- This topic is empty.
-
AuthorPosts
-
2026-10-22 at 4:41 pm #67521
■ 1. Background
AR-C155858 (T14316), CAS: 496791-37-8 is a high-affinity, small-molecule inhibitor of the proton-linked monocarboxylate transporters MCT1 (SLC16A1) and MCT2 (SLC16A7), with inhibition constants of 2.3 nM and 10 nM, respectively. These transporters catalyze the co-transport of monocarboxylates such as lactate and pyruvate together with protons across the plasma membrane, thereby coupling cellular carbon flux to pH homeostasis and redox balance via the lactate/pyruvate and NADH/NAD+ systems [1,2]. In cells where glycolysis generates substantial lactate, MCT1 and MCT2 enable lactate efflux to prevent intracellular acidification, while in cells poised for oxidative metabolism they mediate lactate import for mitochondrial oxidation. Proper trafficking and activity of MCTs depend on ancillary immunoglobulin superfamily proteins (e.g., basigin/CD147 or embigin), which stabilize the transporter at the cell surface and modulate its function [1,2].
By selectively targeting MCT1 and MCT2, AR-C155858 directly modulates this monocarboxylate transport pathway. Inhibition constrains both lactate efflux from highly glycolytic cells and lactate uptake into oxidative partners, collapsing lactate shuttles that normally redistribute carbon and protons between cellular compartments. Functionally, acute exposure to AR-C155858 is expected to increase intracellular lactate and proton load in MCT1/2-dependent cells, shift cytosolic redox toward NADH, and attenuate pyruvate exchange with the extracellular milieu. Conversely, in cells that rely on exogenous lactate as an oxidative substrate, AR-C155858 limits lactate entry and reduces lactate-supported respiration. Because monocarboxylate transport is tightly linked to extracellular acidification and intracellular pH control, blockade by AR-C155858 provides a means to dissect the coordination between lactate transport, carbonic anhydrases, and other pH-regulatory systems during metabolic stress [1,2].
In research workflows, AR-C155858 is well suited for mechanistic interrogation of MCT1/2 contributions to metabolic plasticity. It can be used to: differentiate MCT1/2-dependent versus -independent components of extracellular acidification in real time metabolic flux assays; parse the directionality and magnitude of lactate exchange between co-cultured cell types; and refine isotope tracing experiments by suppressing lactate cycling and exchange, thereby clarifying intracellular labeling patterns from glucose- versus lactate-derived carbons. Its dual activity on MCT1 and MCT2 allows comparative studies of transporter isoform function in systems where both are expressed, while the nanomolar potency enables acute, titratable modulation of flux with minimal off-target confounds expected at low concentrations. Because MCTs are integral to bioenergetic coupling across tissues—including muscle, brain glia–neuron networks, endothelial and stromal compartments—AR-C155858 provides a precise tool for mapping how lactate transport shapes cell–cell metabolic interactions, redox poise, and proton handling across the monocarboxylate transporter pathway [1,2].
■ 2. Literature review
■ 2.1 Responsive nanoparticles modulating microglia lactate transport alleviate M1-type polarization and neuroinflammation for brain injury therapy.
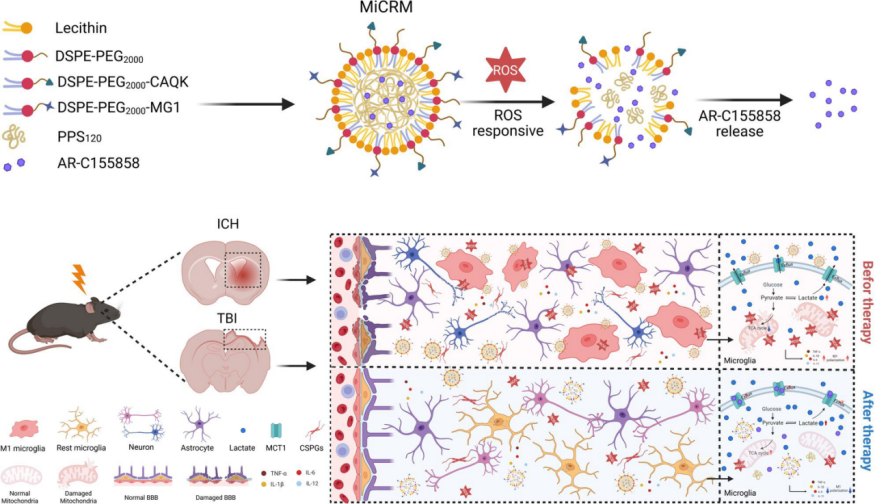
▲ Schematic of MiCRM nanoparticles for ICH and TBI treatment via ROS-responsive release of AR-C155858. (A) The nanoparticle, composed of DSPE-PEG2000 (decorated with CAQK and MG1 peptides), Lecithin, PPS120, and the loaded AR-C155858, disintegrates and releases AR-C155858 in response to the ROS-enriched microenvironment. After therapy, microglia reverse from pro-inflammatory M1 type (red) to resting state (yellow), decreasing levels of TNF-α, IL-1β, and other inflammatory cytokines, reducing lactate transport (MCT1), thereby restoring neuronal mitochondrial function and improving blood-brain barrier (BBB) integrity and neural structure.
AR-C155858 (T14316) is identified as a monocarboxylate transporter 1 (MCT1) inhibitor in this study, as stated in the development of ROS-responsive nanoparticles that co-deliver AR-C155858 with a PPS core. The work reports that these nanoparticles demonstrated controlled release behavior that effectively protected AR-C155858 from enzymatic degradation. Pharmacokinetic analysis revealed that free AR-C155858 was rapidly cleared from circulation, whereas AR-C155858 encapsulated within nanoparticles showed a markedly slower clearance rate, indicating that encapsulation protected the compound from serum elimination and prolonged its systemic retention. Further, surface modification of the nanoparticles with CAQK or MG1 targeting peptides led to an even slower clearance rate of AR-C155858 in serum. Distribution studies in brain injury models demonstrated that the nanoparticle system effectively targeted lesion areas and M1-polarized microglia, enabling efficient delivery of AR-C155858 to microglia. Together, these findings establish the role of the nanoparticle platform in safeguarding AR-C155858 against enzymatic degradation, enhancing its systemic persistence, and promoting its efficient microglial delivery in the context of intracerebral hemorrhage and traumatic brain injury models.[3]
■ 2.2 Structure-guided screening identifies Tucatinib as dual inhibitor for MCT1/2.
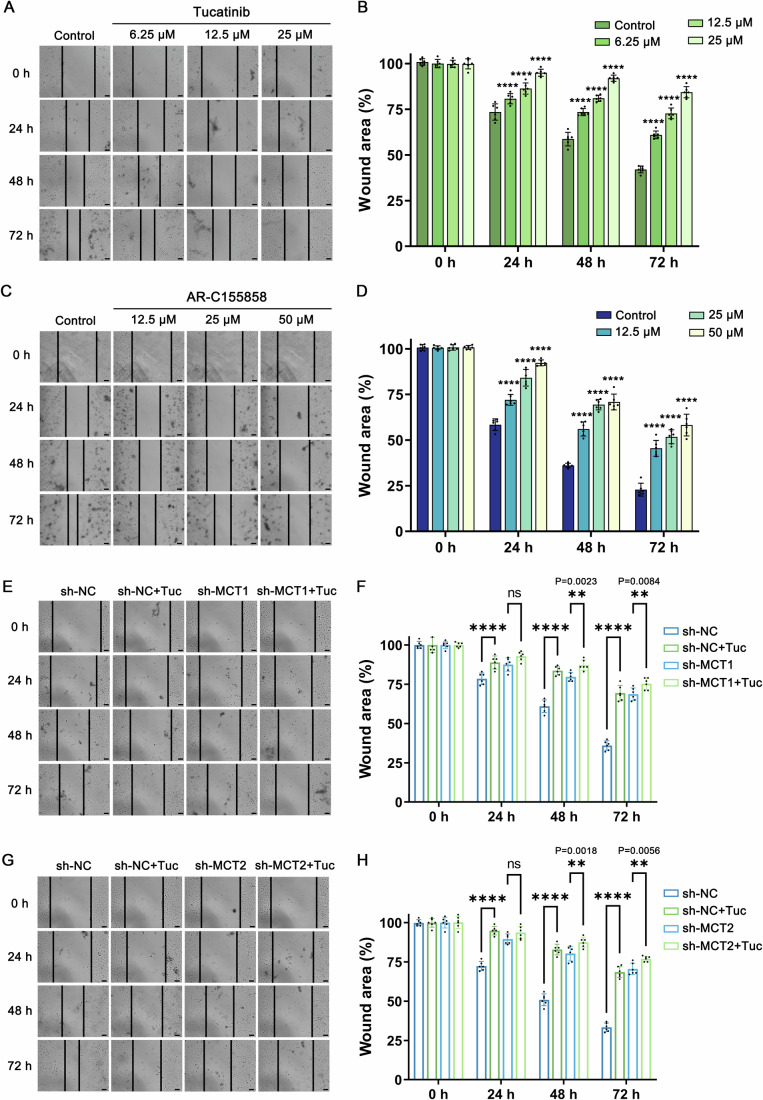
▲ Tucatinib inhibits the migration of HeLa cells by targeting MCT1/2. (A-B) Inhibitory effects of different concentrations of Tucatinib on HeLa cell migration and their quantification, showing that Tucatinib dose-dependently reduces the wound area. (C-D) Using the known MCT1/2 inhibitor AR-C155858 as a positive control, different concentrations also significantly inhibited HeLa cell migration in a dose-dependent manner. (E-H) Comparison of migration inhibition after knocking down endogenous MCT1 or MCT2 and treating with Tucatinib, indicating that knockdown of MCT1/2 significantly enhances the inhibitory effect of Tucatinib on cell migration.
AR-C155858 (T14316) is described as a dual inhibitor of MCT1 and MCT2. Direct binding was measured by bio-layer interferometry to both MCT2-embigin and MCT1-Basigin-2. Functionally, in cells co-expressing MCT2-embigin and a pyruvate sensor, the pyruvate uptake signal significantly decreased after pre-incubation with AR-C155858, demonstrating inhibition of transport. Structural analyses show that AR-C155858 is buried in a large pocket formed by the N-terminal and C-terminal domains of MCT2, with both hydrophobic and hydrophilic residues contributing to recognition. A resolved cryo-EM structure of the MCT2-embigin–AR-C155858 complex, together with docking, revealed a closely matching binding conformation. Molecular dynamics simulations indicated a stable complex with low RMSD values for both the protein and AR-C155858. Energy decomposition identified Y34, F262, D293, R297, and F351 as key residues stabilizing the ligand. At the interaction level, the thienopyrimidine-2,4-dione core is anchored by Y34, Y70, F258, R297, and F351, with R297 forming hydrogen bonds to the 4-carbonyl; the pyrazol ring fits a hydrophobic pocket formed by P37, K38, L66, F262, and I265; and the oxazolidine ring engages S154 and P155, with its 4-hydroxyl hydrogen-bonding to D293. Side chains of K38 and F262 reposition to avoid clashes with AR-C155858. The ligand adopts a Y-shaped arrangement of three rings that are well resolved, and the MCT2-embigin conformation remains essentially identical in the presence of AR-C155858 with sub-angstrom superposition.[4]
■ 2.3 Modulation of Pyruvate Export and Extracellular Pyruvate Concentration in Primary Astrocyte Cultures.
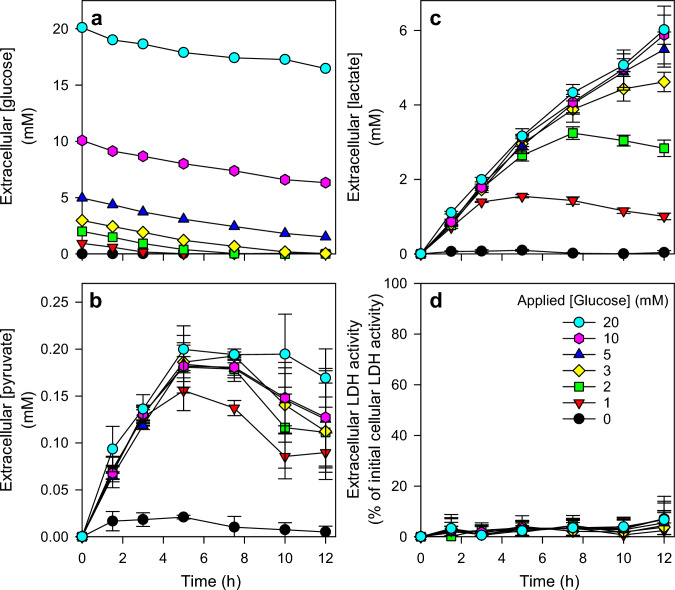
▲ (a) Time courses of extracellular glucose concentrations during a 12-h incubation in buffers containing the indicated initial glucose concentrations (0–20 mM, see legend in d). (b) Changes in extracellular pyruvate concentrations at different glucose levels, showing rapid accumulation peaking at 4–6 h under sufficient glucose (≥5 mM), whereas almost no release occurs under low or no glucose conditions (0–1 mM). (c) Changes in extracellular lactate concentrations at different glucose levels, indicating that lactate production highly depends on initial glucose availability and accumulates over time. (d) Extracellular LDH activity as an indicator of potential cell viability loss, revealing negligible LDH release across all groups, ruling out cell rupture as the cause of metabolite release.
AR-C155858 (T14316) was applied as a monocarboxylate transporter 1 inhibitor in cultured astrocytes. Astrocyte cultures were incubated with 5 mM glucose in the absence or presence of 10 µM AR-C155858, and after 5 h glucose consumption and the concentrations of extracellular pyruvate and lactate were determined, alongside extracellular LDH activity. Under these conditions, AR-C155858 lowered cellular glucose consumption and lactate production by around 40%. AR-C155858 also significantly reduced extracellular pyruvate concentration by around 80%, and extracellular pyruvate accumulation was strongly inhibited. Consistent with these findings, treatment with AR-C155858 lowered glucose consumption and lactate release. When AR-C155858 was co-applied with the mitochondrial pyruvate carrier inhibitor UK5099, the strong effects observed for the individual inhibitors on extracellular pyruvate concentration were eliminated. These data collectively indicate that AR-C155858 decreases glycolytic output measures and markedly suppresses the buildup of extracellular pyruvate in this astrocyte model under defined glucose conditions.[5]
■ 2.4 Inhibition of lactate transport by MCT-1 blockade improves chimeric antigen receptor T-cell therapy against B-cell malignancies.
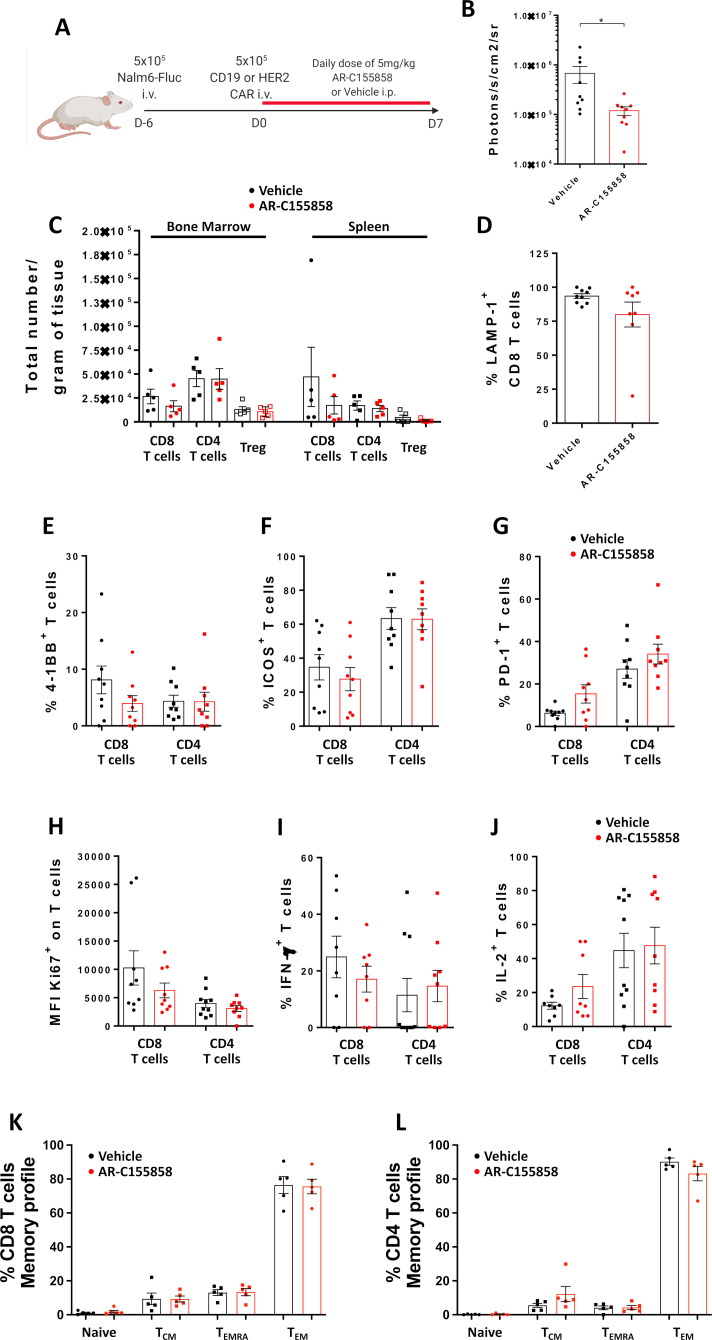
▲ CAR T cells phenotype is unaffected after MCT-1 inhibition (AR-C155858) on a B-cell leukemia xenograft model. (A) Schematic of the experimental design: NOD/SCID mice inoculated with NALM-6 tumor cells were intravenously administered anti-CD19 CAR T cells, followed by daily intraperitoneal injections of AR-C155858 or vehicle for 7 days. (B) Bioluminescence imaging showing that AR-C155858 treatment significantly reduced tumor burden (photons/s/cm²/sr). (C) Total numbers of CD8+ T cells, CD4+ T cells, and Tregs in the bone marrow and spleen showed no significant differences between groups. (D-J) Flow cytometry analysis of bone marrow-infiltrating T cells indicated that AR-C155858 treatment did not alter the expression of functional/activation markers (LAMP-1, 4-1BB, ICOS, PD-1), proliferation capacity (Ki-67), or effector cytokines (IFN-γ, IL-2). (K-L) The distribution of memory subsets (Naive, TCM, TEMRA, TEM) in CD8+ and CD4+ T cells remained consistent between the two groups, unaffected by AR-C155858.
AR-C155858 (T14316) was used in this study as a small-molecule inhibitor of monocarboxylate transporter-1. Direct evidence shows that MCT-1 inhibition with AR-C155858 induced CAR T-cell metabolic rewiring, indicating that the compound actively modulated CAR T-cell bioenergetics. The study also reported that AR-C155858 blocks MCT-2, identifying an additional transporter target for this molecule within the monocarboxylate transporter family. In vivo experimental procedures included systemic delivery of AR-C155858, with the compound administered by daily intraperitoneal injections at 5 mg/kg in a 10% DMSO-PBS vehicle. Together, these findings establish that AR-C155858 was applied to inhibit MCT-1 in the context of CAR T-cell investigations, produced measurable metabolic reprogramming in CAR T cells, and has activity against MCT-2. The dosing regimen details provide the experimental context for its use in animal studies. The combination of these observations supports the study’s focus on leveraging AR-C155858 to modulate lactate transport via MCT-1 during CAR T-cell–related experiments and documents the specific administration approach used to deploy the compound in vivo, alongside its defined biochemical activity on both MCT-1 and MCT-2. The reported metabolic rewiring of CAR T cells following exposure to AR-C155858 represents the key functional outcome directly attributed to this inhibitor in the experimental work.[6]
■ 3. Conclusion
AR-C155858 is a potent small-molecule inhibitor that selectively targets the proton-linked monocarboxylate transporters MCT1 and MCT2, blocking their role in co-transporting lactate and pyruvate with protons across the plasma membrane. This inhibition disrupts lactate efflux from glycolytic cells and lactate uptake by oxidative cells, thereby altering intracellular proton load, redox balance, and pyruvate exchange. Key findings include the compound’s nanomolar affinity for MCT1 and MCT2, structural elucidation of its binding mode within MCT2, and its efficacy in modulating metabolic fluxes in various cellular models such as astrocytes and CAR T cells. Applications demonstrated include enhanced delivery via nanoparticles for brain injury therapy, metabolic reprogramming in immune cells, and refined isotope tracing studies. Future research could focus on leveraging AR-C155858 to dissect metabolic coupling in complex tissue environments, develop targeted delivery systems, and explore its therapeutic potential in metabolic diseases and immunotherapy.
■ 4. Q&A
Q1: What is the primary molecular target of AR-C155858 and how does it function?
A1: AR-C155858 primarily targets the proton-linked monocarboxylate transporters MCT1 and MCT2, inhibiting their function of co-transporting monocarboxylates such as lactate and pyruvate together with protons across the plasma membrane, thereby modulating cellular carbon flux, pH homeostasis, and redox balance.
Q2: How has AR-C155858 been applied in research models according to the text?
A2: AR-C155858 has been applied in multiple research contexts including controlled delivery via ROS-responsive nanoparticles to treat brain injury by targeting microglia, metabolic flux modulation in astrocyte cultures to reduce glycolytic output and extracellular pyruvate, and in CAR T-cell studies to induce metabolic rewiring by inhibiting MCT1 and MCT2.
Q3: What structural insights about AR-C155858 binding to MCT2 are described?
A3: Structural analysis revealed AR-C155858 binds within a large pocket formed by the N-terminal and C-terminal domains of MCT2, involving both hydrophobic and hydrophilic residues such as Y34, F262, D293, R297, and F351. The ligand adopts a Y-shaped conformation stabilized by hydrogen bonds and hydrophobic interactions, with molecular dynamics simulations confirming complex stability.
■ 5. Reference
[1] Halestrap AP. The SLC16 gene family—structure, role and regulation in health and disease. Mol Aspects Med. 2013;34(2-3):337-349.
[2] Halestrap AP, Meredith D. The SLC16 monocarboxylate transporter family. Pflugers Arch. 2004;447(5):619-628.
[3] Ma Y, Chen G, Xu P, Wang B, Teng T, Zheng Y, et al.. Responsive nanoparticles modulating microglia lactate transport alleviate M1-type polarization and neuroinflammation for brain injury therapy.. Journal of nanobiotechnology. 2026;24(1):.
[4] Xu B, Zhou X, Shan Y, Shi S, Li J, Liang Q, et al.. Structure-guided screening identifies Tucatinib as dual inhibitor for MCT1/2.. EMBO reports. 2026;27(3):677-703.
[5] Denker N, Dringen R. Modulation of Pyruvate Export and Extracellular Pyruvate Concentration in Primary Astrocyte Cultures.. Neurochemical research. 2024;49(5):1331-1346.
[6] Lopez E, Karattil R, Nannini F, Weng-Kit Cheung G, Denzler L, Galvez-Cancino F, et al.. Inhibition of lactate transport by MCT-1 blockade improves chimeric antigen receptor T-cell therapy against B-cell malignancies.. Journal for immunotherapy of cancer. 2023;11(6):.
http://www.targetmol.com
TargetMol Chemicals Inc. -
AuthorPosts

- You must be logged in to reply to this topic.